Pages

Friday, August 8, 2014

ESA2014 preview: External chemical defenses in plants

I'll be presenting this at 1:30 PM on Wednesday in the Plant-Insect Interactions II session in the Compagno room. Fellow GGE student and collaborator Billy Krimmel will follow soon after with an interesting talk on tarweeds. 

I've been studying chenopods and their salt bladder system - which is important both physiologically and defensively for the plant - for awhile and with some gentle nudging from my committee, I've been trying to place the chenopod system into a broader context. Namely, what ecologically and evolutionarily differs between a plant which sequesters its chemical defenses (alkaloids, tannins, etc.) in its tissues and one which secretes them onto plant surfaces?

Glandular trichomes (secretory and non-secretory) cover the surfaces of Trichostema laxum.
Coming from New England, where plants with copious exudates are less common, the summer in California is a bonanza of sticky, oily, slimy (!) and otherwise exudate-covered plants. Is this pattern driven by rainfall? Many of these species have congeners elsewhere without copious exudates (e.g. Trichostema, Lessingia, etc.), which begs the question: are exudates effective defenses only in arid environments? Are the defenses liable to environmental removal?

I therefore set up a series of experiments examining these questions. In one, I simulated rain on individuals in a population of Atriplex rosea - a chenopod with defensive exudates - while holding other individuals as controls and rainfall controls (which received water at the base, not on the leaves) and assessed herbivory at the end of the season. Perhaps unsurprisingly, I found a significant increase in herbivory in the group which received rainfall, suggesting that instead of helping these arid, water-starved plants, the rainfall and subsequent removal of exudates (which are entirely water-soluble in A. rosea) actually increased its susceptibility to herbivores.

Chenopods with external defenses (Atriplex prostrata and rosea) and without (Chenopodiastrum murale) at my field site.
Come to my talk to hear more!


Saturday, June 28, 2014

Polymorphic flowers - cool natural history observations

I've been spending as much time in the field (at McLaughlin reserve, which I can't say enough good stuff about) as I can manage lately - trying to complete all the projects I've begun. A quick update on some interesting stuff.

This guy greeted me yesterday morning. Western rattlesnake, Crotalus viridis.
Not sure about the bunny - but maybe a juvenile jackrabbit?


The exudates of Trichostema laxum - also known as turpentineweed or bluecurls - are rather strange smelling (like herbaceous vinegar) and seem to be very deterrent to herbivorous insects in lab trials. So I have a large scale exudate removal experiment going, that while taking up a huge amount of time, seems to be going really well.

Trichostema laxum. You can even see the exudates shining on the leaves!
I am seeing an increase in herbivory (haven't crunched the numbers, but it is noticeable) in the exudate-removed plants, and hopefully, I'll be able to show a fitness effect. However, I wanted to be able to say that any fitness effect was due to herbivory, not differential pollination. So I've been spending 6 or so hours a day watching pollinators visit these plants. Which is also going well, but sitting for that long in the heat is driving me crazy. So I've been taking breaks and visiting other populations of T. laxum to look for herbivory.

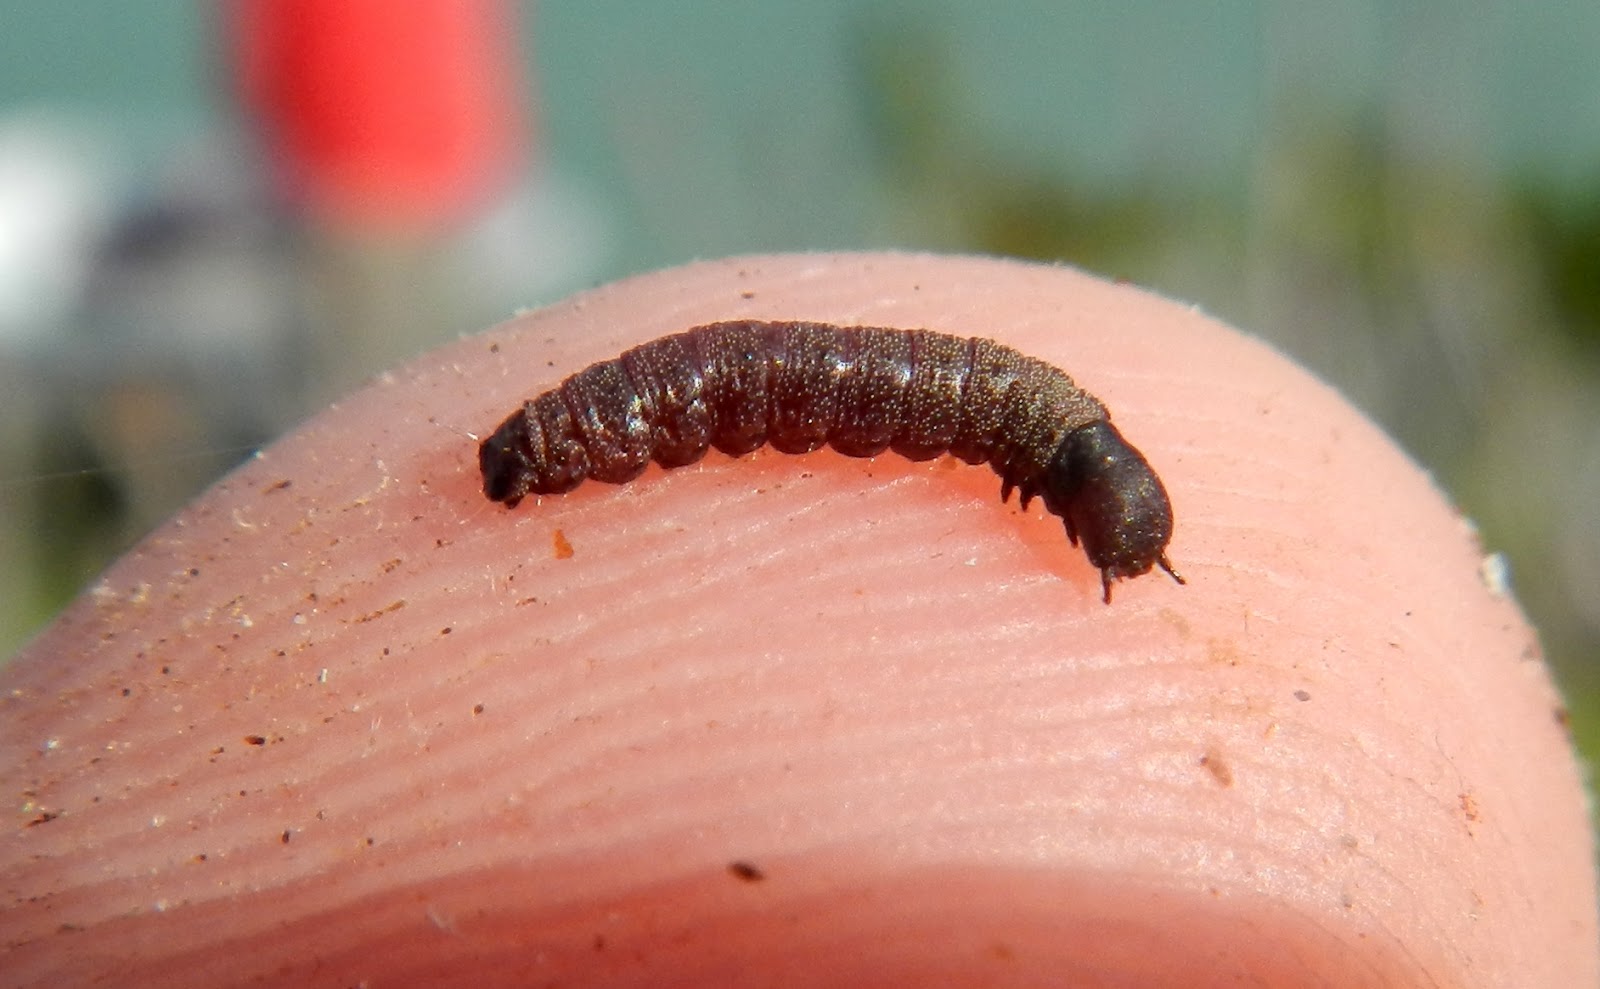
All populations suffer some herbivory, but one population is getting annihilated by this leafhopper and
some noctuid caterpillar!
While scouting populations, I've come across some flower polymorphisms that apparently haven't been described for the species. They occur in low frequency (1:1,000-100,000 depending on the population), but occur nonetheless, and therefore, are interesting. Are they selected against heavily? Or with big populations, are they just swamped out as neutral?


The top left is the "normal" morph - a purple flower which varies a small amount in shade, but not too much. The pink morph is in at least two populations in low frequency and probably exhibits a different molecular structure of anthocyanin - the pigment that gives most plants a reddish or pinkish color. The bottom right plant lacks anthocyanin entirely, it has no reddish parts, including the stem that is reddish in all other individuals of the species. The bottom left has anthocyanin - probably the same form as the normal, and has dark reddish stems - but lacks it on the flowers except on the lower lip.

I'm not sure what to make of these, but I've been gathering fitness data (the anthocyanin-less morph seems to be sterile) and pollination data and I'll hopefully collect seed and do some breeding experiments.

Otherwise, life has been good!

Ctenucha sp. (rubroscapus/multifaria group, I do believe) which is all over the Stachys flowers here. 

Friday, December 20, 2013

A Caterpillar Mystery in the Bahamas

I've been in the Bahamas for the last two weeks, studying the effect of resource pulses (hurricane-wrecked seaweed) on island communities with this project. In doing so, we kept coming upon these strange shelters on wild guava (Psidium longipes), locally called Bahama stopper, since the hard wooded bush/tree would apparently stop any progress you try to make into the thick coppice.

What on earth is this? ~  4 cm tall (pretty damn big by insect standards).
Inside some of these shelters (2/13), there was an odd larva, apparently a beetle larva, or so I initially thought. Because I am mostly a caterpillar person, I didn't really pay it much mind. 

A really terrible picture, but notice the "antennae". About 2-3 cm long. 

Louie, while processing insect samples one night, noticed that some things were not right about the apparent beetle larva - namely it had prolegs, the fleshy appendages that give caterpillars the appearance of having more than the six legs all insects have. I then looked at the "antennae" and found that they were not segmented, a dead giveaway that this was, in fact, a caterpillar and the "antennae" were actually tentacles (yes, that is the technical term for the fleshy projections that many caterpillars have - monarchs for instance).

Several of the shelters were torn like this, suggesting predation (by a bird [?]). This was the
only shelter with lines affixing it at the top - many had lower lines. 

I got much more interested after that, and sent along these pictures to Charley Eisemann, a good friend and probably the person on earth with the most knowledge about insect shelters. His blog - linked above - is simply phenomenal and if anyone was going to know the answer, he would. Very quickly (within a few minutes), he had correctly found the family of the moth - Mimallonidae. The amazing part here is that Charley has never seen a member of this family! Mimallonidae is an extremely small family by Lepidoptera standards, ~200 spp. - only 3 of which occur regularly in the US, a fourth is described from the US in Brownsville, TX, but is probably a tropical stray. He even dug pretty deep and found a very likely species identity, Ciccinus packardii - known from Cuba and known to feed on other Psidium species. While I do not know this for sure, it seems that is the most likely candidate as the larva matches very well the few images of Ciccinus online, and less so the other mimallonid genera. 

After a bit more searching, we came upon a young larvae feeding in a leaf press on P. longipes, which was not what I expected. This family is known as the "sack-bearers" and I was expecting something more along the lines of a bagworm (Psychidae), instead of a leaf presser.

A young (2nd, 3rd instar?) larva of this Ciccinus sp. ~ 8mm
Which brings us to the strange, pitcher plant-like shelters. The larva is oriented vertically inside the shelter, with a strange butt plate plugging up the bottom hole and the head just below the upper hole. What function the little hood forms is mysterious - perhaps shading the larva from the hot Bahamian sun or fierce rains? The better-known Ciccinus species of the US, C. melshiemeri, feeds on old oak leaves (too tannic for most caterpillars) and constructs a shelter, sort of like the pictured ones of frass pellets, silk and oak leaves in which it spends the winter as a larva, prior to pupation in the spring. This seems to be the case for this species as well - in two cases, I found spent pupal skins.

Spent pupal skin (successful emergence!) inside one of the shelters. You can also see the construction of silk and what
appears to be finely ground frass (caterpillar poop - a common building material for cats). 
Interestingly, I did find one that fit the description of the C. melshiemeri shelters well.

This was the only shelter anchored into leaves (it was vacant, unfortunately). You can see well the frass pellets forming the top of the shelter here.
The same shelter, with a Psidium leaf forming one side. 
These guys kept me occupied for quite awhile (I even dreamt about them!) and seem like a worthy avenue for future rearing efforts... there are a great deal of questions that remain about the shelters: Why the strange shape with a hood? Why build a free standing shelter, as opposed to anchoring it to a stem like most moths? Why wait around in a shelter instead of pupating right away? Do the shelters protect inhabitants from predators and parasitoids?


perhaps the prettiest of all found. I like the subtle banding.

Many thanks to Charley, Julia Blyth, John De Benedictus, Louie Yang, Jonah Piova-Scott and Jenn Mckenzie (who was the only one that could find occupied shelters) for help with the identification and finding of these guys.

Wednesday, December 4, 2013

Chenopod salt bladders

I recently published a paper on a cool plant defense system of certain plants in the Chenopodiaceae.

Three chenopod species at my field site (McLaughlin Reserve, Lake County, CA). In the center the whitish plant is Atriplex rosea, in the front and front left the dark green plant is Chenopodiastrum murale and in the back left the plant with triangular leaves is Atriplex prostrata
The chenopods are a diverse "family" (people can't really agree whether they are their own family or form a family with the amaranths) found worldwide. They tend to be common in three habitats, dry, salty shrublands, saltmarshes and recently disturbed areas (often roadside or agricultural). Two genera form most of the diversity and have many economically-important species in them. The first is Atriplex, the saltbushes (used to refer to perennial species) or oraches (used to refer to annual species).

A sea of Atriplex prostrata at McLaughlin. 

The second is Chenopodium, which includes the food species quinoa (C. quinoa) and lambs-quarters or pigweed (C. album).

Chenopodium neomexicanum, in the greenhouse

The coolest thing about these plants (and certain other chenopods - but not spinach or beets), in my opinion, is that they have these strange bladder cells on their leaf and stem surfaces. Several scientists have studied the salt sequestration of these bladder cells and found they are extremely important in ionic balance of the plant in saline environments. But many, if not most, of the bladdered chenopods are not halophytes (plants which live in salty areas). So what else are these good for?

The leaf of a cultivated variety of Chenopodium album. All the purple balls are salt bladders - the leaf surface below is green. 

I suspected, given their location on the plant surfaces, that they might be part of a defensive system of the plant, as they would be the first tissues contacted by herbivores and they would allow the plant to segregate defenses, which are often bad for the plant, away from photosynthetic tissues. So I tested the defensive function of these bladders by removing them from leaves and testing herbivore preference with a choice, assessing herbivore preference without a choice, and removing them in the field and assessing herbivory rates compared to control leaves.


Removed bladders from the C. album leaf above. The purple coloration is due to betalain, a compound shown in other studies of amaranths (closely related) to be an effective defense against insect herbivores. 

I found strong support for a defensive function for these structures. Plants have all sorts of cool structures (domatia, hairs, sticky glands, etc.) which are defensive in function and with this work, I added one more to this list. I'm working on a few further projects on chenopods now, I'll update with those when they get completed.

Reference: LoPresti, EL (2013) Chenopod salt bladders deter insect herbivores. Oecologia, DOI: 10.1007/s00442-013-2827-0

Saturday, November 30, 2013

Fall 2013

A really busy, but awesome fall, condensed.

Spent most of my time looking at, growing, weighing, dissecting, caressing, keying, watering, fertilizing, pressing and reading/writing about chenopods.

Atriplex sp. fruiting bracts. This is probably A. rosea, though the bracts are longer and rounder than any other
A. rosea I have run into recently. 

However, I got in some wonderful camping in the mountains with friends (and the new old truck!).

Camping with the new old truck!


Where we found a few mushrooms. Some edible.


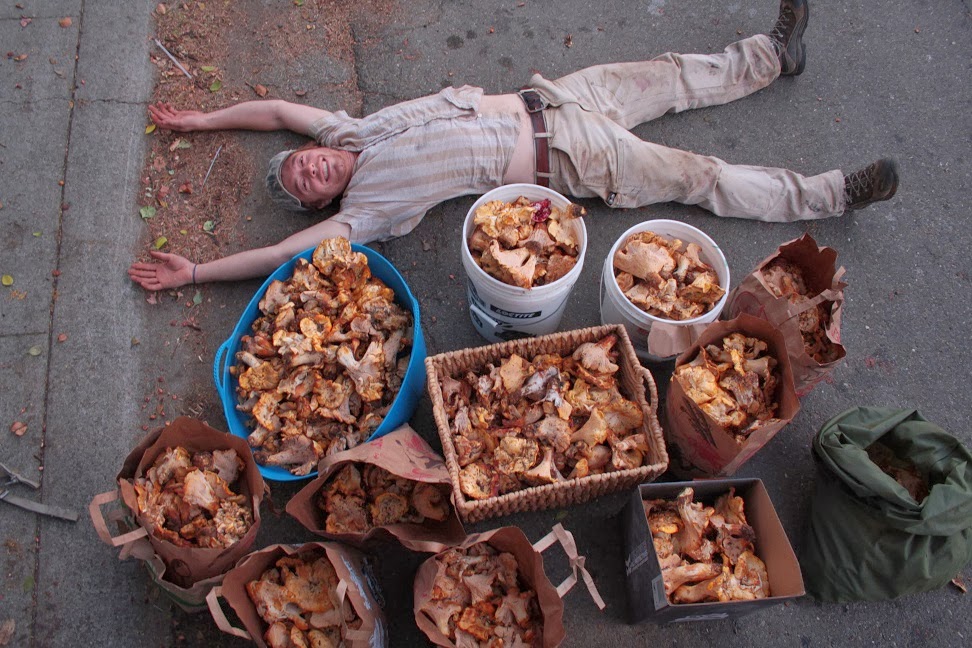
We ate chantarelles for awhile (3 meals a day for basically weeks). 

Found one lion's mane mushroom (Hericium erinaceus).

And some not:


Scaly chantarelle, Gomphus flocossus


I even took a trip home, where I learned how to differentiate the plumages of adult and 2nd winter Ring-billed Gulls (among all sorts of wonderfulness of being in New England in November and seeing family and friends). 


2nd winter Ring-billed Gull. Note the uniformly dark primaries without white spotting. Also the blueish legs and bill.

2nd winter, in front, with two adults, behind. 


I'm about to depart on all sorts of adventures (Bahamas! Jordan and Israel!), I'll update this again at some
point.